Coral reefs
This article describes the habitat and functions of coral reefs. It is one of the sub-categories within the section dealing with biodiversity of marine habitats and ecosystems.
Contents
- 1 Introduction
- 2 Formation (warm water corals)
- 3 Distribution
- 4 Biology
- 5 Reef zonation (WWC)
- 6 Conditions for reef growth
- 7 Sediment transport
- 8 Coral reef ecosystem
- 9 Threats
- 10 Climate change impact on coral reefs
- 11 Coral reef restoration and creation
- 12 Related articles
- 13 External link
- 14 References
Introduction

Coral reefs are among the most diverse ecosystems in the world. Corals belong to the Phylum Cnidaria. The best-known type of corals is the one living in clear, warm tropical waters with plenty of colorful fishes (Fig.1). This is a rocky, shallow water type. The water is clear because concentrations of nutrients are typically low. Besides, there are also deep water corals that live in dark cold waters and soft corals that live in shallow, cold waters. Coral reefs are wave-resistant carbonate structures built primarily by reef-building corals, together with other calcifying organisms such as coralline algae. Coral reefs provide the physical foundation of a number of mid-ocean atoll nations (e.g., Kiribati, Tuvalu, Maldives, and Marshall Islands). Coral reefs also protect coral islands and island populations against the destructive forces of the sea under storm conditions, see Coral islands.
Formation (warm water corals)
The formation of corals begins when free-swimming coral larvae attach to submerged rocks (e.g. sinking volcanic islands) or other hard substrate along the edges of islands or continents. Over time, different reef types may emerge, which can be classified as fringing reefs, barrier reefs and atolls. Their development depends on the interaction between reef accretion, antecedent topography, relative sea-level change and subsidence or uplift.
Atolls are circular or oval coral reefs (Fig. 2a) that partially or completely encircle a lagoon. A barrier reef (Fig. 2b) is a reef that borders the shoreline over a long distance. They are separated from the adjacent land mass by a lagoon. A fringing reef (Fig. 2c) forms borders along the shoreline and the surrounding islands, but at shorter distance than barrier reefs. It is directly attached to the land. Darwin's classical subsidence model explains the transition from fringing reef to barrier reef and atoll around subsiding volcanic islands, but not all reefs follow this evolutionary sequence.
More detailed classifications distinguish special reef arrangements such as apron, patch, ribbon, table and bank reefs. Apron reefs are very similar to fringing reefs. Both are extending downward from the land margin, the former more gently sloping than the latter. Patch reefs (Fig. 2d) are small, isolated outcrops of coral surrounded by sand and/or seagrass, and may form part of a fringing reef system. Ribbon reefs (Fig. 2e) are the small and long components of a barrier or are connected to an atoll lagoon. Table reefs can evolve into future atolls, but are not yet connected to a lagoon. Finally, bank reefs resemble the patch reefs, but are larger and often semi-circular.
Coral reefs are among the oldest habitats in the ocean. They have slow growth rates and it may take up to 10,000 years for a coral reef to fully develop from the first colonizing larvae [2]. The different types of coral reefs all share similarities in their biogeographic profiles. Horizontal and vertical zonation depends on bottom topography, depth, wave and current strength, light, temperature and suspended sediments.
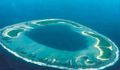
Fig. 2a. Atoll reef
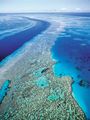
Fig. 2b. Barrier reef
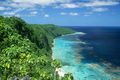
Fig. 2c. Fringing reef
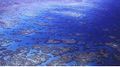
Fig. 2d. Patch reef
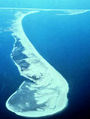
Fig. 2e. Ribbon reef


Distribution
Warm water corals (WWC)
The warm water corals are found in the tropics (between 30°N and 30°S, Fig. 3) in areas where the water is clear and over 18°C. Consequently, corals are typically absent along the western margins of Africa and South America where cool water upwelling prevails. The maximum depth for warm water corals is generally around 60 meters. Some species of coral are found in all the world's oceans. Tropical coral ecosystems cover about 300,000 km2 of the Earth’s surface.
Cold-water corals (CWC)
Globally, cold-water corals (CWC) cover a wide range of depths (40 - 2000 m), water temperatures of 4-10 °C and latitudes (70°N – 60°S, Fig. 3). They are most common on continental slopes, on deep shelves and along the flanks of oceanic banks and seamounts, and are found around vents, in fjords and around offshore submarine banks (Cordes et al., 2016[3]). Submarine canyons are hotspots of cold-water corals by providing exposed hard and steep substrate and strong bottom currents that transport organic matter from the continental shelf to the deep sea[4]. The majority of CWCs occur between depths of 200 to 1000 m, with the bathymetric ranges becoming shallower towards the poles (Roberts et al., 2009[5]).
Desmophyllum pertusum (formerly Lophelia pertusa) (Fig. 8) is the dominant reef-forming CWC in the Atlantic (Hebbeln et al., 2020[6]). The suitable temperature ranges from 4°C to 13°C, but they occur in some regions at much higher temperatures (>20°C). Desmophyllum is not found in the polar regions. Desmophyllum can tolerate surprisingly low oxygen concentrations (lower oxygen limit DO ~4 ml/l but in some areas ~1 ml/l) and locally forms thriving reefs under hypoxic conditions in waters saturated with aragonite (Hebbeln et al, 2020[6]). The other important reef forming cold water coral, the fragile zigzag coral Madrepora oculata, is found in the north-east and western Atlantic and the Mediterranean Sea. Gorgonians (soft corals) are a major cold water species in the South China Sea[7].

Biology

The principal reef-building organisms are hard coral (scleractinian corals). The formation starts with a larva known as planula that settles down and attaches itself to a hard substrate. Then the larva develops into a coral polyp and secretes calcium carbonate around its body. The reproduction is by budding, an asexual process. As the asexual reproduction continues, the colony grows. Some polyps in the colony develop gonads and are able to reproduce sexually. These polyps release sperm and eggs in the surrounding water. To help with fertilization, both eggs and sperm cells have protein molecules on their surfaces to identify other cells of the same species (Karleskint, 1998[9]).

The coral polyp has a sac-like structure that is protected by a rigid calcium-carbonate exoskeleton (Fig. 4). This is called a corallite. The bottom of the corallite is divided into vertical segments or septa. At the top, the polyp has an opening that is a combined mouth and anus. This leads to the gut. The opening is surrounded by tentacles with mucus secreting cells for catching prey. The photosynthetic dinoflagellates symbionts commonly called zooxanthellae, giving the coral its color, live within cells of the coral gastrodermis (Fig. 5). This provides a stable environment for them. The cells are abundant and can represent 5-15% of the tissue weight[10]. The zooxanthellae require sunlight for photosynthesis. They transfer photosynthetically fixed organic carbon and other metabolites to the coral host. This makes the conditions for the formation of skeletons more suitable. In turn, the zooxanthellae get a suitable habitat.
Not all corals are reef building species. There are also hard corals existing as single, solitary polyps. Some temperate species form small colonies only. Corals that lack the hard outer covering of calcium carbonate are soft corals. Cold water reef-building corals generally lack the symbiotic dinoflagellates and obtain their energy heterotrophically.
Reef zonation (WWC)

On the seaward side, the reef rises from the lower depths of the ocean to a level just at or just below the surface of the water (Fig. 6). This is called the reef front or fore-reef. The slope of this zone varies from gentle to steep. It sometimes forms a vertical wall known as a drop-off. But generally, the reef front forms finger-like arrangements called spur and groove formations. It breaks the wave energy and prevents damage to the reef. The grooves are sand-filled pockets, which allow sediment to be channelled down and away from the coral surface and provide a habitat for many species of burrowing organisms. The reef crest is the highest point of the reef. More land inward, the reef flat or back reef is formed. This zone has a high variability. The bottom of the reef flat consists of rock, sand, coral cobble or a combination of these. Seagrasses are commonly found in this zone. The reef ends at the shoreline or descends into the lagoon.
A typical Caribbean reef zonation is illustrated by the following species. On the on the intermediate slopes of the reef front, dome-shaped, massive brain corals (Diploria, Fig. 7a) and columnar pillar corals (Dendrogyra, Fig. 7b) are found. Below this region, plate corals such as Pectinia, Pavona and Agaricia are found. Higher upon the reef, where wave stress is greatest, there are branched species of coral. A coral occuring in this zone is the elkhorn coral (Acropora palmata, Fig. 7c). Behind the reef front, more protected zones are occupied with more delicate species such as the staghorn coral (Acropora cervicornis, Fig. 7d). In shallow, calmer waters away from the reef front, small species such as rose (Meandrina, Manicina), flower (Mussa, Eusmilia) and star (Montastraea) corals are found. [9]
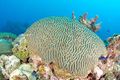
Fig. 7a. Brain coral (Diploria strigosa) [11]
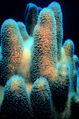
Fig. 7b. Pillar coral (Dendrogyra cylindrus) [12]
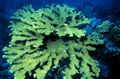
Fig. 7c. Elkhorn coral (Acropora palmata)
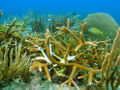
Fig. 7d. Staghorn coral (Acropora cervicornis) Photo credit W. Jaap


Conditions for reef growth
Warm water corals
Reef-building, warm water corals generally prefer the following environmental conditions for optimal growth:
- Clear water, allowing light to reach the photosynthetic zooxanthellae. Light-absorbing adaptations enable some species to live in dim blue light.
- Ocean temperatures above 18°C; the optimum temperature for most corals is 26–27 °C. Many coral species only survive within a narrow temperature window.
- Sufficient water motion to supply food and oxygen, disperse larvae and prevent excessive sediment accumulation on the reefs.
- Sufficiently high pH to prevent aragonite dissolution; ocean acidification can cause loss of reef structure.
- Hard substrate.
Coral reefs are generally absent from river mouths that have characteristically low salinity levels and high sediment supply. Corals thrive in low-nutrient waters; high-nutrient levels can severely inhibit coral production[13].
Cold water corals

Cold water corals (CWCs) are organisms belonging to the cnidarian orders Scleractinia (stony corals), Alcyonacea (soft corals, including gorgonians), Antipatharia (black corals), Pennatulacea (seapens) as well as the hydrozoan family Stylasteridae (hydrocorals) [15]. Cold water corals do not need light to function. They obtain their nutrients and energy completely from trapping plankton and organic particles in passing currents. Desmophyllum pertusum has been shown to incorporate everything from dissolved and particular organic carbon to algal biomass to small zooplankton.
Although the majority of the species-level diversity is in the solitary corals, some of the CWC (e.g. Desmophyllum pertusum) form extensive reef structures, occasionally accumulating into large carbonate mounds, or bioherms (Cordes et al., 2016[3]). These reefs function as refuges, feeding areas and nurseries for many species, including commercially important fish[16]. CWC reefs are also linked to a high biodiversity.
CWCs are fragile and vulnerable to physical disturbance. The polyps cannot escape disturbances and their structures are brittle. They also grow slowly (there are no zooxanthellae in the dark), so it takes a long time to rebuild the reef when it is damaged. A further disadvantage is that they cannot respond to fast-occurring changes in their environment, as they are adapted to stable conditions (WWF, 2001[17]). Trawl gear can damage CWC communities by reducing or changing coral abundances, diversity and community or the removal of structuring species.
Carbonate balance
The persistence and growth of a coral reef depend on its carbonate balance. Carbonate is produced mainly by reef-building corals and calcifying algae, with additional contributions from other calcifying organisms. Production is opposed by bioerosion through grazing and boring organisms, chemical dissolution and physical erosion. The resulting carbonate material can remain incorporated in the reef framework, become cemented, be broken down into sediment and rubble, or be transported within or away from the reef. Reef accretion therefore depends not only on net carbonate production but also on sediment and rubble retention or import, cementation, physical erosion and sediment export.[18]
Studies of coral reef accretion rates suggest that contemporary reef accretion rates are lower than past long-term rates (Holocene averages). Explanations put forward are recent widespread loss of coral cover and relative stability of sea levels for much of the mid- to late-Holocene, thus limiting shallow-water accommodation space for more recent vertical reef accretion (Woodroffe and Webster, 2014[19]). Whether modern rapid rates of sea level rise may reinvigorate vertical accretion in such locations remains uncertain.
Sediment transport
Wave transformation on a coral reef is strongly influenced by the shape of the reef platform and therefore differs from wave transformation on a sandy shore (discussed in Shoreface profile). Two key differences are the steep outer slope of the reef platform (fore-reef slope) and the nearly horizontal, shallow platform (the rough reef flat and sandy back reef zone, see Fig. 6) in front of the beach. Sea swell waves break on the fore-reef slope and lose additional energy on the reef flat. In the wave transformation process, energy is transferred from high-frequency waves to low-frequency (infragravity) waves. The low-frequency waves can be further amplified if their frequency is close to the resonance frequency of the reef platform. Such resonance enhances flooding risks (Gawehn et al., 2016[20]).
As the broken swell waves propagate across the reef flat, they become skewed (wave orbital velocities are stronger in shoreward than in seaward direction) and forward-leaning asymmetric (wave orbital accelerations in shoreward direction are higher than in seaward direction). Wave skewness and asymmetry favor shoreward over seaward bed load sediment transport, see Shoreface profile. Infragravity waves that dominate on the back of the reef flat contribute mainly to suspended sediment transport, which is also predominantly shoreward (Pomeroy et al., 2015[21]). Wave transformation processes on the reef platform therefore cause reef-derived coral sand to be brought to the island shore.
Coral reef ecosystem
Many coral reefs, particularly those surrounded by nutrient-poor oceanic waters, sustain high productivity through efficient retention and recycling of nutrients and organic matter. Dissolved and particulate organic matter produced within the reef is processed by microorganisms and other reef organisms and thereby retained within the food web. Microbial decomposition regenerates inorganic nutrients, while sponges can take up dissolved organic matter, including coral-derived organic matter, and convert part of it into particulate detritus that becomes available to other reef organisms.[22][23]
Coral reefs provide a structured habitat with niches for many species. Branching and massive corals, cavities, crevices and the underlying carbonate framework create a complex three-dimensional environment used for shelter, feeding and reproduction by fishes and many invertebrates. This holds both for warm-water and cold-water reefs. Faunal biomass can be orders of magnitude above that of the surrounding area. Loss of structural complexity therefore affects considerably more than coral abundance alone.
A diverse coral-associated fauna depends on the host coral on which they live as epibionts, either as surface encrusting epifauna or by living partially embedded in the coral skeleton. This symbiotic relationship can be either facultative, where the symbiont can survive without the host, or obligatory, where the associate cannot exist without the host or inversely (e.g. Zooxanthellae). Some epibionts provide protection from predators and disease or provide cleaning services, while others can wound their hosts (e.g., boring mussel Leiosolenus spp.), impede growth or completely suffocate the host. High densities of some symbiont taxa can be harmful to the host coral if skeletal integrity is compromised or if too many polyps are damaged. High densities of symbionts (e.g., coral barnacle Pyrgomatidae, Christmas tree worm Spirobranchus spp., Leiosolenus spp.) can occur under influence of eutrophication[24].
Grazing fishes and sea urchins remove algae from reef surfaces and can help maintain substrate available for coral recruitment. When herbivory is strongly reduced, fleshy macroalgae can proliferate and interfere with coral recruitment and growth, although the strength of coral–algal competition varies among reefs and conditions.
Many animals of the warm-water reefs are sessile or move very slowly. Sponges are found at deeper parts of the reef front. Smaller animals are found in the waters behind the reef. Anemones remain fixed in one place by a muscular, mucus-secreting basal disk. If the conditions become unfavorable, some sessile species can release themselves and crawl over the bottom, searching for a more suitable area. Fanworms or featherduster worms are represented by two families: the serpulid worms (Fig. 9a), which produce tubes of calcium carbonate, and sabellid worms, which form tubes of sand and small particles pasted together by mucus.
Organisms that can often be found on the branches of coral reefs are: fish (Fig. 9b), crustaceans, starfish, molluscs, brittle stars (Fig. 9c), sea pens (Fig. 9d), sea urchins and squids. Sponges, bryozoans, hydroids, and some other coral species are found on the coral itself. The octopus (Fig. 9e) is one of the most formidable predators. It can rapidly change its color in response to its background (camouflage) and has very sharp eyesight. Octopuses have the ability to squeeze through small spaces where potential predators cannot gain access. Moray eels are among the nocturnal predators of reef fishes and invertebrates. During the day, predatory fishes such as groupers, snappers, jacks and barracudas (Fig. 9f) occupy higher trophic levels. (Karleskint, 1998[9]).
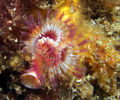
Fig. 9a. Serpulid worm (Serpula columbiana)
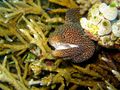
Fig. 9b. Moray eel
Fig. 9c. Brittle star
Fig. 9d. Sea pen. Photo credit NOAA.
Fig. 9e. Common octopus (Octopus vulgaris) [25]
Fig. 9f. Barracuda (Sphyraena barracuda). Photo credit NOAA.


Threats
Natural causes are:
- Tropical cyclones, storms and tidal emersions..
- El Niño: change of sea surface temperatures outside the tolerance range of the local coral species.
- Predation by fishes, marine worms, barnacles, crabs, snails and sea stars.
- Dust outbreaks.
Human-induced causes are:
- Chemical pollution: see the article Threats to Coral Reefs: the Effects of Chemical Pollution.
- Eutrophication: Many eutrophicated regions which in the past were renowned for their corals are now dominated by macro algae and filamentous algae and expansion of seagrass beds (Bell, 1992[26]).
- Fishery: Coral is easily damaged by fishing gear, especially bottom trawls. Even worse are destructive fishing practices, such as cyanide and dynamite fishing, which are still prevalent in poorly regulated and enforced maritime areas in Southeast Asia.
- Dredging and dumping: Direct cutting through the reef and release of plumes of suspended sediment, which can settle on coral reefs and damage them from food and sunlight starvation.
- Coral mining: Extraction of coral for use as a building material.
Climate change impact on coral reefs
Until now, the above human activities were the main cause of the widespread decline of coral reefs. In addition to these local human pressures, coral reefs are increasingly affected by climate change, in particular by rising seawater temperature and ocean acidification. Of all coastal ecosystems, coral reefs are globally the most threatened by the effects of climate change (Ani and Robson, 2021[27]). A strong relationship has been observed between short periods of elevated sea temperature (heat waves), mass coral bleaching and mortality within warm-water coral reefs (Hoegh-Guldberg, 1999[28]). There is also strong experimental evidence that net ecosystem calcification and net community production will be altered when concentrations of dissolved CO2 in seawater increase (Noonan et al., 2018[29]; Comeau et al., 2019[30]; Doo et al., 2019[31]).
However, field observations show that after severe bleaching by a heat wave, corals exhibit a greater tolerance to a similar successive event (Pratchett et al., 2013[32]; Guest et al. 2012[33]; Thompson and Woesik 2009[34]; AIMS, 2026[35]). Howells et al. (2025[36]) attribute increased tolerance to standing genetic variation in fitness-related traits in reef-building coral populations and strong selective pressure imposed by marine heatwaves. The increase in thermal tolerance is estimated at about 0.1°C per decade, which is slightly less than the 1990-2020 global warming trend (Lachs et al., 2023[37]). However, the trend in thermal tolerance may not be consistent across colonies within and among coral reefs (Denis et al., 2024[38]), nor consistent across ocean basins (Whitaker and DeCarlo, 2024[39]). There is no evidence yet that the bleaching tolerance of coral reef systems can keep pace with global warming if the global warming trend persists or accelerates. Besides, while global warming is a major component of global change, it is not the only factor. Other stressors for coral reefs that must be considered include ocean acidification, sea-level rise, deoxygenation, cyclones, pollution as well as numerous biotic pressures such as diseases, pest species, and overfishing (Klein et al., 2024[40]).
Coral reef restoration and creation
Coral reefs are very effective wave attenuators under storm conditions, besides offering an essential habitat for many marine organisms. Coral restoration can locally accelerate recovery of coral cover, habitat complexity and reef functions, particularly where the causes of degradation have first been reduced. Restoring degraded coral reefs can be an advantageous alternative to artificial coastal protection structures. Promising results have been achieved with techniques involving coral gardening as intermediate step, where fragmented or recruited corals are grown in sheltered sites before transplantation to natural habitats (Young et al., 2012[41]). Substrate for new reefs can be created in a suitable environment with artificial materials, e.g. rock-filled steel baskets (Reguero et al., 2018[42]) serving as support for colonization by corals. Extension of coral reefs has been experimented with success by transplanting corals on a substrate of artificial reefs (Perkol-Finel and Benayahu, 2009[43]).
However, present restoration techniques operate at scales far smaller than current global reef loss and cannot by themselves compensate for reef degradation driven by continued ocean warming. Restoration should therefore complement, rather than replace, climate mitigation and management of local pressures (Mula et al. 2025[44]).
Related articles
External link
References
- ↑ http://en.wikipedia.org/wiki/Coral_reef
- ↑ Barnes R.D. 1987. Invertebrate Zoology. Fifth edition. Fort Worth, TX. Harcourt Brace Jovanovich College Publishers. 92-96, 127-134, 149-162
- ↑ 3.0 3.1 Cordes, E., Arnaud-Haond, S., Bergstad, O-A., Costa Falcao, A.P., Fereiwald, A., Toberts, J.M. and Bernal, P. 2016. The First Global Integrated Marine Assessment, World Ocean Assessment, Chapter 42. Cold-Water Corals. Regular Process for Global Reporting and Assessment of the State of the Marine Environment. UN
- ↑ De Leo, F. C., Smith, C. R., Rowden, A. A., Bowden, D. A. and Clark, M. R. 2010. Submarine canyons: hotspots of benthic biomass and productivity in the deep sea. Proc. R. Soc. B Biol. Sci. 277: 2783–2792
- ↑ Roberts, J.M., Wheeler, A.J., Freiwald, A. and Cairns, S.D. 2009. Cold-water Corals: The Biology and Geology of Deep-sea Coral Habitats. Cambridge: Cambridge University Press
- ↑ 6.0 6.1 Hebbeln, D., Wienberg, C., Dullo, W-C., Freiwald, A., Mienis, F., Orejas, C. and Titschack, J. 2020. Cold-water coral reefs thriving under hypoxia. Coral Reefs 39: 853–859
- ↑ Ta, K., Song, X., Wei, Z., Du, M., Xu, H., Chen, S., Li, J., Liu, S. and Peng, X. 2024. Oasis of the deep: Cold-water corals of the South China Sea. Marine Environmental Research 195: 106354
- ↑ UNEP/GRID-Arendal - Hugo Ahlenius
- ↑ 9.0 9.1 9.2 Karleskint G. 1998. Introduction to marine biology. Harcourt Brace College Publishers. p.378
- ↑ Kemp, D.W., Kempf, S.C. and Fill, W.K. 2020. The weight of it all: symbiotic dinoflagellates in Caribbean reef‑building corals Marine Biology 167, 121
- ↑ http://nl.wikipedia.org/wiki/Hersenkoraal - Photo credit Albert Kok
- ↑ http://en.wikipedia.org/wiki/Dendrogyra - Photo credit NOAA
- ↑ Kench, P.S. and Owen, S.D. 2022. Coral Systems. Ch. 8.22 of Treatise on Geomorphology (ed. Shroder, J.F.), Elsevier
- ↑ Roberts, J.M. 2012. Changing Oceans Expedition 2012, funded by UK Ocean Acidification programme (NERC, DECC, Defra)
- ↑ Cairns, S. D. 2007. Deep-water corals: an overview with special reference to diversity and distribution of deep-water scleractinian corals. Bull. Mar. Sci. 81: 311–322
- ↑ Roberts, J. M., Wheeler, A. J. and Freiwald, A. 2006. Reefs of the deep: the biology and geology of cold-water coral ecosystems. Science 312: 543–547
- ↑ WWF. 2001. Cold water corals: fragile havens in the deep. p. 12
- ↑ Lange, I.D., Perry, C.T. and Alvarez-Filip, L. 2020. Carbonate budgets as indicators of functional reef “health”: A critical review of data underpinning census-based methods and current knowledge gaps. Ecological Indicators 110: 105857.
- ↑ Woodroffe, C.D. and Webster, J.M. 2014. Coral reefs and sea-level change. Marine Geology 352: 248–267
- ↑ Gawehn, M., van Dongeren, A., van Rooijen, A., Storlazzi, C.D., Cheriton, O.M. and Reniers, A. 2016. Identification and classification of very low frequency waves on a coral reef flat. J. Geophys. Res.: Oceans 121: 7560–7574
- ↑ Pomeroy, A.W.M., Lowe, R.J., Van Dongeren, A.R., Ghisalberti, M., Bodde, W. and Roelvink, D. 2015. Spectral wave-driven sediment transport across a fringing reef. Coast Eng. 98: 78–94
- ↑ Nelson, C.E., Wegley Kelly, L. and Haas, A.F. 2023. Microbial Interactions with Dissolved Organic Matter Are Central to Coral Reef Ecosystem Function and Resilience. Annual Review of Marine Science 15: 431–460.
- ↑ de Goeij, J.M., van Oevelen, D., Vermeij, M.J.A., Osinga, R., Middelburg, J.J., de Goeij, A.F.P.M. and Admiraal, W. 2013. Surviving in a marine desert: the sponge loop retains resources within coral reefs. Science 342: 108–110.
- ↑ van der Schoot, R.J. and Hoeksema, B.W. 2022. Abundance of coral-associated fauna in relation to depth and eutrophication along the leeward side of Curaçao, southern Caribbean. Marine Environmental Research 181, 105738
- ↑ http://en.wikipedia.org/wiki/Octopus - Photo credit Albert Kok
- ↑ Bell, P.R.F. 1992. Eutrophication and coral reefs—Some examples in the Great Barrier Reef Lagoon. Water Research 26: 553–568
- ↑ Ani, C.J. and Robson, B. 2021. Responses of marine ecosystems to climate change impacts and their treatment in biogeochemical ecosystem models. Marine Pollution Bulletin 166, 112223
- ↑ Hoegh-Guldberg, O. 1999. Coral bleaching, climate change and the future of the world’s coral reefs. Mar. Freshw. Res. 50, 839–866. doi: 10.1071/MF99078
- ↑ Noonan, S.H.C., Kluibenschedl, A. and Fabricius, K.E. 2018. Ocean acidification alters early successional coral reef communities and their rates of community metabolism. PLoS ONE 13(5): e0197130
- ↑ Comeau, S., Cornwall, C. E., DeCarlo, T. M., Doo, S. S., Carpenter R. C. and McCulloch, M. T. 2019. Resistance to ocean acidification in coral reef taxa is not gained by acclimatization. Nature Climate Change volume 9: 477–483
- ↑ Doo, S.S., Edmunds, P.J. and Carpenter, R.C. 2019. Ocean acidification effects on in situ coral reef metabolism. Nature Scientific Reports 9:12067 https://doi.org/10.1038/s41598-019-48407-7
- ↑ Pratchett, M. S., McCowan, D., Maynard, J. A. and Heron, S. F. 2013. Changes in bleaching susceptibility among corals subject to ocean warming and recurrent bleaching in Moorea, French Polynesia. PLoS One 8: 1–10
- ↑ Guest, J. R., Baird, A.H., Maynard, J.A., Muttaqin, E., Edwards, A.J., Campbell, S.J., Yewdall, K., Affendi, Y.A. and Chou, L.M. 2012. Contrasting patterns of coral bleaching susceptibility in 2010 suggest an adaptive response to thermal stress. PloS One 7: 1–8
- ↑ Thompson, D. M. and Van Woesik, R. 2009. Corals escape bleaching in regions that recently and historically experienced frequent thermal stress. Proc. R. Soc. B Biol. Sci. 276: 2893–2901
- ↑ AIMS 2026. Great Barrier Reef annual summary report Coral reef condition 2025-2026. Australian Institute of Marine Science
- ↑ Howells, E.J., Abrego, D., Schmidt-Roach, S., Puill-Stephan, E., Denis, H., Harii, S., Bay, L.K., Burt, J.A., Monro, K. and Aranda, M. 2025. Marine heatwaves select for thermal tolerance in a reef-building coral. Nat. Clim. Chang. 15: 829–832
- ↑ Lachs, L., Donner, S.D., Mumby, P.J., Bythell, J.C., Humanes, A., East, H.K. and Guest, J.R. 2023. Emergent increase in coral thermal tolerance reduces mass bleaching under climate change. Nature Communications 14, 4939
- ↑ Denis. H., Bay, L.K., Mocellin, V.J.L., Naugle, M.S., Lecellier, G., Purcell, S.W., Berteaux-Lecellier, V. and Howells, E.J. 2024. Thermal tolerance traits of individual corals are widely distributed across the Great Barrier Reef. Proc. R. Soc. B 291, 20240587
- ↑ Whitaker, H. and DeCarlo, T. 2024. Re(de)fining degree‑heating week: coral bleaching variability necessitates regional and temporal optimization of global forecast model stress metrics. Coral Reefs 43: 969–984
- ↑ Klein, S.G., Roch, C. and Duarte, C.M. 2024. Systematic review of the uncertainty of coral reef futures under climate change. Nature Communications 15, 2224
- ↑ Young, C. N., Schopmeyer, S. A., and Lirman, D. 2012. A review of reef restoration and coral propagation using the threatened genus Acropora in the Caribbean and Western Atlantic. Bul. Mar. Sci. 88: 1075–1098
- ↑ Reguero, B.J., Beck, M.W., Agostini, V.N., Kramer, P. and Hancock, B. 2018. Coral reefs for coastal protection: A new methodological approach and engineering case study in Grenada. Journal of Environmental Management 210: 146-161
- ↑ Perkol-Finkel, S. and Benayahu, Y. 2009. The role of differential survival patterns in shaping coral communities on neighboring artificial and natural reefs. Journal of Experimental Marine Biology and Ecology 369: 1–7
- ↑ Mula, C., Bradshaw, C.J.A., Cabeza, M., Manca, F., Montano, S. and Strona, G. 2025. Restoration cannot be scaled up globally to save reefs from loss and degradation. Nature Ecology & Evolution 9: 822–832
Please note that others may also have edited the contents of this article.
|


